Showing posts with label Human Evolution. Show all posts

Tuesday, January 17, 2012

Animal Cognition & Consciousness (II): Metacognition & Mentalizing


As I wrote in my last post, three kinds of behaviours are most often discussed in debates about animal consciousness and cognition:
“1. Mirror self-recognition
2. Tests of metacognition;
3. Metacognition of others’ mental states” (Gómez 2009: 45)
After having discussed the first capacitiy in my previous post, I will discuss the latter two in this post, starting with metacognition, that is being aware of one’s own knowledge states, and then turn to being aware of other’s mental states.

Metacognition.

Being aware of one’s own mental states, i.e., reflective consciousness, surely seems to be one of the most crucial components of self-awareness. In one paradigm used to test for metacognitive awareness, monkeys were trained to select, out of a number of two or more images, the one that is identical to an image they have been shown earlier. As is to expected, the monkeys’ performance progressively deteriorated the longer the delay was between the sample image and the selection task.

Sunday, January 8, 2012

Animal Cognition & Consciousness (I): Mirror Self-Recognition

Darwin made a mistake. At least that is what Derek Penn and his colleagues (2008) claim in a recent and controversial paper in Behavioral and Brain Sciences. Darwin (1871) famously argued that the difference between humans and animals was “one of degree, not of kind.”

This, according to Penn et al. is of course true from an evolutionary perspective, but in their view,
“the profound biological continuity between human and nonhuman animals masks an equally profound discontinuity between human and nonhuman minds” (Penn et al. 2008: 109).
They hold that humans are not simply smarter, but human cognition differs fundamentally and qualitatively from that of other animals.

One pervasive proposal is that we do not simply possess a unique set of cognitive capacities, but that it might be consciousness itself that is uniquely human as well, a view that goes back at least to Descartes (Burkhardt & Bekoff 2009: 41). However, there are also many scholars and researchers who agree that there is evidence for higher-order cognition in nonhuman animals ( ‘animals’ after this) and that they might possess at least some degree of consciousness (Burkhard & Bekoff 2009: 40f.).

In this and my next post, I will write about three kinds of phenomena that are most often discussed in debates on whether animals have some form of higher-order cognition and consciousness or not: self-awareness, awareness of one’s own cognitive states, and awareness of others’ cognitive states and intentions.

Monday, November 15, 2010

Michael Tomasello - Why We Cooperate

cross-posted at Replicated Typo

In this post I will offer a short overview of some aspects of Michael

Tomasello’s latest book „Why We Cooperate,” which is based on his 2008 Tanner Lectures on Human Values.

Tomasello deals with the question howcooperative behaviour and itssocio-cognitive foundations arise both in development and during theevolution of the human species. His short text is accompanied by four short commentaries by leading scholars who contributed in important ways to the theory of the evolution and ontogenetic development Tomasello espouses here. These are: psychologist Carol S. Dweck, anthropologist Joan B. Silk, philosopher Brian Skyrms and developmental psychologist Elizabeth Spelke.

In this post I only want to briefly summarize some of the key tenets of Tomasello’s book to offer an introduction to his work on cooperation, whose main impetus it is to have a closer look at the relatively simple and primal cooperative and interactive social behaviour that builds the foundation of human culture.

The Uniqueness of Human Culture

Tomasello points out that a lot of social animals can be said to have a culture insofar as the same animal species can live in slighty different habitats and show different behaviours (e.g. chimpanzees of different regions have different pant-hoots, many species have regionally differing techniques for obtaining food).
In this regard, human culture is only quantitatively different from that of, say, the other great apes. The difference here is that humans simply have to learn about more culture-specific behaviours and artefacts. The principle however, is the same.
But according to Tomasello, there are two aspects that also make human culture also qualitatively different from all others:

  1. human culture is cumulative. That is, artefacts and behavioural practices often become more complex over time. Every improvement or accepted changed will be transferred to the next generation and so forth.
  2. human culture is unique in that there are social institutions, which create and enforce culture norms and practices.

What underlies these two features “are a set of species-unique skills and motivations for cooperation.” (Tomasello 2009: XIII) on which Tomasello elaborates in the subsequent chapters.

Early Spelke

In the first chapter, “Born (and Bred) to Help”, Tomasello outlines how children come to be (or already are) cooperative so that they can take part in an co-establish human culture.
He advances a theory he dubs “Early Spelke, Later Dweck.”Research done by Tomasello and many others shows that by the time they are about one year old, infants already prove to be cooperative and helpful in many contexts. In addition, these tendencies seem not be taught but come naturally to them given sufficient interaction with a normal environment. (Hence ‘Early Spelke, referring to the work done by Harvard psychologist Elizabeth Spelke on innate or naturally emerging ‘core knowledge’).

Later Dweck
Later in development however, this picture becomes more complex: children come to be concerned about whether others will reciprocate and also about how they are judged by others in the group. They also gradually internalise cultural norms.
Up to now Tomasello has mostly described the initial starting point from which children refine their social behaviour and become truly cultural beings. More precisely, what happens is that children become less ‘indiscriminate’ in terms of who they behave altruistically towards, but become more discerning based on a variety of characteristics.

This phase could be described as the birth of the ‘public self’ which is concerned with ‘impression management.’ The child comes to realize that

“they are targets of the judgements of others who are using social norms as standards.” (Tomasello 2009: 31).

In other words, for the first time they develop a larger we- or group perspective, which is connected to the insight that this ‘we-ness’ is tied to certain social norms (‘They way we do things’).

Experiments show that by the age of three children actively follow social norms and also already participate in enforcing these norms.
If they grasp how a game works, for example, not only do the play it according to the rules, but they also correct others and object if they try to play the game differently.

Interestingly, they also use ‘normative declaratives’ like “One can’t do that” or “It doesn’t work like that,” when doing so.

Those findings contrast sharply with Jean Piaget’s influential view of how social norms are internalised. According to him, (and building on the work of Piaget, moral psychologist Lawrence Kohlberg), children follow social norms only because they fear punishment.

Instead, from and early age on children already seem to adopt some kind of ‘view from nowhere’ (Nagel 1970) and a “he is me” attitude of identification when interacting with others (see also Meltzoff 2005).

As Tomasello argues,

"without this added dimension of some kind of ‘we’ identity and rationality , it is impossible to explain take it upon themselves to actively enforce social norms on others from a third-party stance, especially those norms that are not based on cooperation but rather on constitutive rules that are, in an important sense, arbitrary" (Tomasello 2009: 39).

For Tomasello these processes form the basis of human cooperative behaviour, cultural transmission, social institutions and cultural practices.

References:

Meltzoff, Andrew N. (2005): Imitation and other minds: The "Like Me" hypothesis. In S. Hurley and N. Chater (Eds.), erspectives on Imitation: From Neuroscience to Social Science. Vol. 2, pp. 55-77). Cambridge, MA: MIT Press

Nagel, Thomas (1970) The possibility of altruism. Princeton, NJ: Princeton Unviersity Press.

Tomasello, Michael (2009): Why We Cooperate. Cambridge, MA/London, England: Boston Review.

Friday, September 3, 2010

Is 'Shared Intentionality' the Foundation of Human Uniqueness?


Wow, I can't believe that it's been two months since I last posted anything. But I'm still working on my last term papers and preparing for writing my state examination thesis (similar to a master's thesis), so I rarely find any time to blog.
But I've been meaning to repost a blog post I wrote over at replicated typo - where I've become a contributor - about the concept of "shared intentionality" (see e.g. Tomasello & Carpenter 2007). So here it is:

Shared or collective intentionality is the ability and motivation to engage with others in collaborative, co-operative activities with joint goals and intentions. (Tomasello et al. 2005). The term also implies that the collaborators’ psychological processes are jointly directed at something and take place within a joint attentional frame (Hurford 2007: 320, Tomasello et al. 2005).


Michael Tomasello and his colleagues at the Max-Planck-Institute for Evolutionary Anthropology in Leipzig, Germany have proposed that shared intentionality and the cognitive infrastructure supporting it may be the crucial feature that makes humans unique.

(You can hear Michael Tomasello talk about shared intentionality in his brief 2009 acceptance speech for the prestigeous "Hegel-Price" here. Transcript here)

Understanding Pointing

The infrastructure of this capacity requires abilities that are present in humans at a surprisingly young age. Although human children only know what other can see and what the cannot see at 24 months of age (Moll & Tomasello 2006). other social cognitive skills appear at a much earlier date. (Chimpanzees, interestingly, appear to only know what another one sees only in competitive situations, i.e. when there are two rewards and one of them is in plain sight of a dominant chimpanzee, the sub-dominant chimpanzee takes the one that is hidden from view (Hare & Tomasello 2004).)

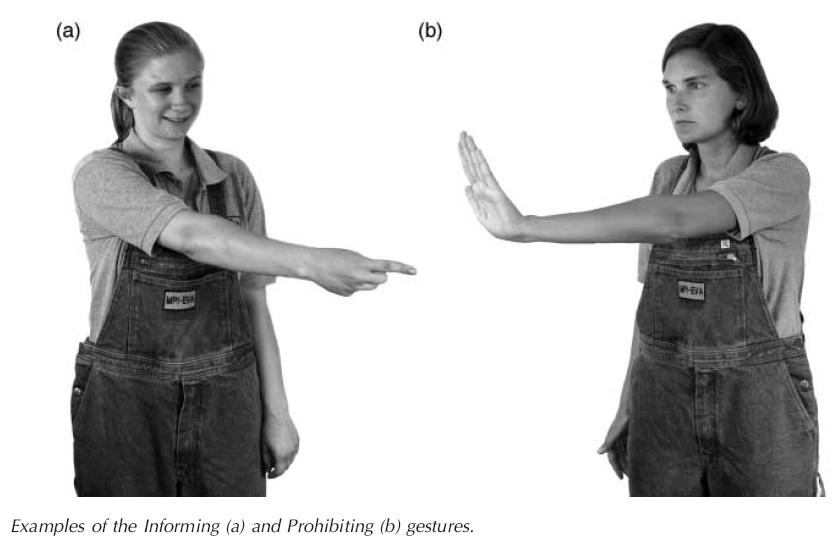
At 14 months of age for example, human children are able to successfully pass an object-choice task. In this task, children are presented with two upside-down buckets, one of which contains a toy, and the experimenter points toward the bucket where the toy is hidden. The child then turns to the right bucket and retrieves the toy. Although this task may appear simple, it is remarkable that chimpanzees fail it. In contrast to children, they fail to see the pointing gesture as a relevant cooperative signal within a shared attentional frame. Instead chimpanzees seem to think something along the lines of: “‘A bucket. So what? Now where’s the food?’ They do not understand that the pointing is intended to be ‘relevant’ to the searching as a shared activity (see Sperber & Wilson, 1986)” (Tomasello & Carpenter 2007: 122).


But this result is reversed in chimpanzees when instead of pointing cooperatively towards the bucket, the experimenter makes a prohibiting gesture by holding her arm out towards the correct container with her palm out, says something like “Don’t take this one” in a firm manner and then leaves the room. In this competitive context chimpanzees can successfully infer where the hidden reward. What is equally interesting is that 24 month old children do not retrieve the hidden toy possibly because they were better at cognitive control than 18 month old children and chimpanzees and were aware of the social and communicative conventions of the prohibiting action (Hermann & Tomasello 2006, see e.g. Miller et al. 2002, Tomasello 2008: 208ff. ).


Understanding Shared Experience

At the age they are able to solve a simple informative object-choice, infants also can keep track of who is familiar with some toy and who is not through shared experience.


In an experiment involving three toys and two experimenters, the first experimenter and the infant played together with two of the toys, then the first experimenter left the room. After that, the second exph the experimenter and the infant played with all three of the toys, but with two of them in a normal fashion and with one of them in a very excited manner. When the first experimenter then came back in ambiguously asked for “it” infants reliably gave them the toy they had an excited shared experience with. Control conditions clearly showed that the infants knew “which of these objects “we”—and not just me or you alone—had experienced in a special way in the immediate past: (Moll et al. 2008: 98). A linguistic experiment in which a mother played with three toys together with her child then left the room, and the child then played with a fourth novel toy together with an experimenter had similar results. When the mother came back and looked at the four toys and excitedly exclaimed “Oh, a modi, a modi!” the child successfully learned this as the word for the fourth novel object drawing on their experience of sharing common ground with the mother in respect to the first three toys, but not with the new toy (Akhtar et al. 1996).

Understanding Joint Commitments

In general, human children and infants seem to be much more interested in cooperation, sharing, and committing themselves to a shared goal and a shared experiential perspectives than other primates. In specific contexts chimpanzees exhibit joint, co-operative, coordinated hunting for small monkeys (Boesch & Boesch 1989), and human-raised enculturated chimpanzees successfully solve co-operative problem-solving tasks in which food could be retrieved only together with a non-competitive, familiar human adult both when it required parallel and complementary roles. When it comes to social games, however, such as one person rolling a ball down and another one catching it with a can (complementary), or making a wooden block jump on a trampoline (parallel), the chimpanzees showed no interested and played with single parts of the game set-up for themselves. 18 to 24 month-old human children on the other hand successfully took part in both the co-operative problem-solving tasks as well as the social games. What is more, in contrast to the chimpanzees the children actively tried to reengage the adult when he ceased doing his part of the co-operative activity in both problem-solving and social contexts. Children thus explicitly displayed skills of shared intentionality by being jointly committed to a shared goal with shared intentions. These skills can also be seen in the manifesting conversational and linguistic skills of children around that time (Tomasello 2003).

Pointing in Human Children and Chimpanzees


The shared intentionality infrastructure is also already present in communicative power of pantomiming and informative pointing just for the sake of sharing attention and sharing information which infants acquire around their first birthdays (Tomasello 2008: 111). These behaviours even include references to absent object or events such as something that is going on outside, happened in the past or will happen again in the future, a cup that is empty and should be filled, to something that is hidden or not present at the moment (Tomasello 2008: 116f.). Chimpanzee’s on the other hand, practically rarely point in natural contexts, and captive chimpanzees only do so when requesting something, using the human as a “social tool” (Tomasello 2006). A similar imperative behaviour has recently been observed in the wild: during grooming, chimpanzees sometimes point to a specific part of their body where they want to be scratched. (Pika & Mitani 2009). These "directed scratches" however, are also imperative in nature and not declarative.

In contrast, 12 to 18 month-olds also point co-operatively to inform others of the location of an object they are looking for. (Liszkowski et al. 2006 : 173). Generally humans infants and children have a natural tendency to be extremely cooperative in a variety of task and help others solve their problems
“even when the other is a stranger and they receive no benefit at all. However, our nearest primate relatives show some skills and motivations in this direction as well, and this suggests that the common ancestor to chimpanzees and humans already possessed some tendency to help before humans began down their unique path of hypercooperativeness.” (Warneken & Tomasello 2006: 1302 )

The evidence presented here strongly suggest that it indeed seems that social intelligence was a driving factor and the crucial foundation for what makes us unique.

But in addition, it seems that in the human lineage the “Machiavellian Intelligence Hypothesis,”, which sees social competition as the main causal factor for primate, including human brain evolution (Byrne & Whiten 1988, Humphrey 1976), does not apply across the board. Instead, it seems that the unique aspects of human cognition were driven, and are maybe even constituted by, collaboration, cooperation and the natural motivation to share experiences, intentions and perspectives, which then led to the advances in culture, technology, and higher-order cognition we see today (Moll & Tomasello 2007).

References:

Akhtar, N., Carpenter, M., & Tomasello, M. (1996). The role of discourse novelty in early word learning. Child Development, 67, 635-45.

Boesch, C. & Boesch, H. (1989): Hunting behavior of wild chimpanzees in the Taï-National Park. American Journal of Physical Anthropology 78(4), 547-573.

Byrne, R. & Whiten, A. (eds) (1988) Machiavellian intelligence: social expertise and the evolution of intellect in monkeys, apes and humans. Oxford, UK: Oxford University Press

Hare, Brian, and Michael Tomasello. (2005). Human-like social skills in dogs? Trends in Cognitive Science, 9, 439-444.

Herrmann, Esther. & Michael Tomasello, (2006). Apes' and children's understanding of cooperative and competitive motives in a communicative situation. Developmental Science, 9, 518-529

Humphrey, N. (1976) The social function of intellect. In Growing points in ethology (eds P. P. G. Bateson & R. A. Hinde), pp. 303–317. Cambridge, UK: Cambridge University Press.

Hurford, James M. (2007): The Origins of Meaning: Language in the Light of Evolution. Oxford: Oxford University Press.

Sperber, Dan and Deirdre Wilson (1995): Relevance: Communication and Cognition. Second Edition. Malden et al.: Blackwell.

Miller, Earl K., David J. Freedman and Jonathan D. Wallis (2002.) “The Prefrontal Cortex: Categories, Concepts and Cognition.” In: Phil. Trans. R. Soc. Lond. B 357: 1123–1136

Moll, Henrike and Michael Tomasello (2006): Level 1 Perspective-Taking at 24 Months of Age. British Journal of Developmental Psychology 24, 603–613

Liszkowski, U., Carpenter, M., Striano, T., & Tomasello, M. (2006). Twelve- and 18-month-olds point to provide information for others. Journal of Cognition and Development 7: 173-187.

Moll, Henrike, & Michael Tomasello. (2007) Co-operation and human cognition: The Vygotskian intelligence hypothesis. Philosophical Transactions of the Royal Society 362: 639-648.

Moll, Henrike., Richter, N., Carpenter, M., & Tomasello, M. (2008). Fourteen-month-olds know what ‘we’ have shared in a special way. Infancy, 13(1), 90-101

Tomasello, Michael (2003): Constructing A Language. A Usage-Based Approach. Cambridge, Massachusetts; London, England: Harvard University Press.

Tomasello, Michael (2008): The Origins of Human Communication. Cambridge, MA; London, England: MIT Press.

Tomasello, Michael and Malinda Carpenter (2007): “Shared Intentionality.” In: Developmental Science 10.1, 121-125.

Tomasello, Michael, Malinda Carpenter, Josep Call, Tanya Behne, and Henrike Moll (2005): Understanding and Sharing Intentions: The Origins of Cultural Cognition. In: Behavioral and Brain Sciences 28:5, 675–691.

Warneken, Felix. & Michael Tomasello, (2006). Altruistic helping in human infants and young chimpanzees. Science, 31, 1301 - 1303.

Sunday, June 13, 2010

Cognigrams

On Thursday I went to a talk by Miriam Noel Haidle, who talked about tool use in human and non-human animals. Haidle is part of the research project "The role of culture in early expansions of humans," which looks extremely interesting.
In her talk, Haidle introduced the idea of "cognigrams," which code the cognitive operations necessary for performing a complex task with multiple steps such as tool use. What is most interesting is that you can create cognigrams for the tool-using behaviour of humans, other tool using animals, and pre-humans, and then compare their complexity and use this to asses their cognitive potential.

Here's the abstract of her most recent paper elaborating on this idea:

"Tool use is the main database to track down behavioral developments in the archaeological record and thus human evolution. Working-memory capacity and modern cognitive potential, however, are no simple and obvious characters in tool behavior. Coded in cognigrams, which allow a direct comparison, animal and human tool use can be examined for specific aspects of the working-memory capacity. Detailed studies of tool behavior of wasps, sea otters, bottlenose dolphins, and chimpanzees are presented and compared with the manufacture and use of Oldowan tools and Lower Paleolithic spears. Although this shows a wide range of problem-solution distances, problem solving in animals seems to be restricted to problem complexes for which a solution can be found in spatial and temporal vicinity. In human evolution, the complexity of tool behavior increases regarding the number of active foci managed at a time in an action, the number and diversity of operational steps in a problem-solution complex, and the spatial and temporal frame in which solutions are sought. The results suggest a gradual development of the different aspects of a complex capacity instead of a late introduction of a closed phenomenon with only different facets."

Haidle, Miriam Noël (2010) Working‐Memory Capacity and the Evolution of Modern Cognitive Potential. Current Anthropology 51:s1, S149-S166

Here are two of these 'cognigrams', one of a chimpanzee tool set which is used to extract termites, (Haidle 2010: S154) and one of the cognitive complexity needed to create the kind of 400,000 year-old spear found in Schöningen, Germany. (Haidle 2010: S156)


Monday, February 8, 2010

Biolinguistics, Cooperation, the Importance of Theory of Mind for Language - and Dinosaurs


Some interesting links:
  • The journal "Biolinguistics" now has a blog (here). On it they want to post "a variety of material pertaining to the field of biolinguistics." As of now there isn't very much content other than some information on conferences but I'll stay tuned.

  • On a related note, Julia Fischer of the Cognitive Ethology Laboratory at the German Primate Center in Göttingen, Germany has written a short review of Michael Tomasello's book "Why We Cooperate." I've written a short summary of the slim volume myself, but I seem to have msiplaced the document... Anyway, this review is by somebody who really knows the stuff and is quite enlightening.

  • Also, over at Babel's Dawn there is an interesting discussion of a paper by David Leavens and Tim Racine (abstract here) that questions whether it is really justified to attribute sophisticated psychological processes to preverbal infants in the way Michael Tomasello and many others do. Instead, they argue that learning and growing up in a human community play a much more important part that is normally acknowledged (first part here, second part here). Edmund Blair Bolles thinks that the argument has some merit but remains sceptical. In the comment section of his first post, the authors themselves weigh in.

  • Lastly, and not really relatedly, I really like this cartoon:
  • hat tip: Richard Beck


Saturday, August 15, 2009

Language, Thought, and Space (V): Comparing Different Species

As I’ve talked about in my last posts, different cultures employ different coordinate systems or Frames of References (FoR) "which serve to specify the directional relationships between objects in space, in reference to a shared referential anchor” (Haun et al. 2006: 17568) when talking about space. As shown in my last post these linguistic differences boil down to certain cognitive differences.
Whether speakers mainly use a relative, ego-based FoR, a cardinal-direction/or landmark-based absolute FoR, or an object-based, intrinsic based FoR, also influences how they solve and conceptualise spatial tasks.

In my last post I posed the question whether there is a cognitive “default setting” that we and the other great apes inherited from our last common ancestor that is only later overridden by cultural factors – and, crucially, which Frame of Reference is might be the default one?


Haun et al. (2006: 16570) argue that
"there has been a great deal of speculation about the inherited structure of spatial relational thought. Immanuel Kant argued that the human body provides the source of our basic intuitions about the nature of space. In agreement, many cognitive scientists hold the assumption that spatial cognition is fundamentally egocentric [references omitted].”
In the same vein, Dirven et al. (2007: 1213), point out that
“The principle of corporeal deixis [i.e. body-based or body-centric spatial reference] is even so self-evident that it has been considered by most linguists, including cognitive linguists, as the default case, if not the universal one (Talmy 1983).”
I myself also thought this way and found Karl Bühler’s (1934) notion of the ego-based “Here-Now-I”-origo quite self-evident. In Bühler’s view, this deictic centre is the origin of a “coordinate system of subjective orientation,” which builds the basis and referential anchoring for all communicative acts and all social interaction and coordination,

However, we can still see the egocentric frame of reference as the universal default case and see absolute frames of reference as being cultural variations that transform our innate frame of reference. This would thus still be in line with the paradigm mentioned above as well as with developmental psychologist Jean Piaget’s central assumption that in cognitive development infants start with an egocentric perspective on the world and only later learns to coordinate multiple perspectives on the world.

To test whether this is really the case, Haun et al. used a similar but simplified setting like in their first experiment that I described in my last post, and tested gorillas, chimpanzees, bonobos, orangutans, and 4-year-old German children.

This time there were only 3 identical cups on the table so the object-centred and the geocentric conditions from the previous experiment were collapsed.
The subject was first shown where a reward is hidden
(X = Cups | = Screen E= Experimenter O=Hidden Object)
and was then rotated 180° and brought to an identical table behind the screen where they could then again locate the reward.

In the Relative condition the reward was in relation to the subject. If it was hidden to his left on table 1 it was also hidden to his left on table 2 :
In the Absolute condition “the hiding and finding cups maintained position Relative to the larger, surrounding environment” and also to “a salient landmark between the two tables, namely the screen or the experimenter” (Haun et al. 2006 : 17569).
It turned out that the great apes including the 4-year old children deployed an allocentric/environment-based layout more readily than an ego/self-based spatial strategy. At the very least, these data indicate that
“Despite common expectations, [...] Hominid spatial cognition is at least not always primarily egocentric“ (Haun et al. 2006: 15751).
To further corroborate this evidence, Haun et al. 2006 tried an even simpler version of this task on the non-human great apes as they are known to have problems with abstract rule-learning and generally scored quite low on the second experiment.

Thus, in a third experiment, the subjects were directed to the first table and in the baseline condition were rewarded for picking a cup no matter which it was for 10 times. The animals were then led to the table that was on the other side of the screen and the experimenter started to only reward one of the cups until the apes consistently picked a particular cup ten out of twelve times in a row. If they had succeeded in doing so, they were redirected to the original table and in the test trials were again rewarded for all of their ten choices.
In this way, the experimenters induced a “response” or “training bias” in the apes: In the test condition they tended to preferably pick the same cup as the one for which they were rewarded 10 times in a row in the training condition. That is, if they were rewarded for picking the middle cup in the training session, they also preferred to pick the middle cup when rotated 180° and brought back to the original table in the test condition.


The interesting question then is: If they were rewarded for picking say this cup:

in the training condition: which cup would they show the response bias for in the test condition? Would they interpret this as being ‘the cup to their left’? Or would they interpret it as being allocentrically/environmentally based?
As in the second experiment, great apes showed a preference for environmental cues as opposed to self-based cues. That is if they developed a preference for the cup in the upper illustration, they then preferred to pick the following cup in the rotated test condition.
Haun et al. (2006: 17572) conclude that gorillas, chimpanzees, bonobos, orangutans, and we all have inherited “preference for allocentric spatial strategies” from our shared ancestor.

“Based on this result, we argue that, at least for small-scale spatial relations, the inherited cognitive mode of operation is not, as argued by Kant and others, egocentric but preferably deploys environmental cues as common reference between object.”
I think this is a fascinating result and I find the argument very convincing. It is also strengthened by findings from cognitive and linguistic development: By 16 months, when they have become successful mobile navigators, children competently use non-egocentric cognitive strategies. 3- to 5-year old English-speaking children even appear to be “better at allocentric strategies than at egocentric ones.” Moreover, in cultures where an absolute frame of reference is the dominant one, children master “this system as early as 4 and certainly by 7 years of age.” Children who live in cultures that dominantly employ a relative frame of reference, on the other hand, do not seem to master the full use of a left and right system until about 11 years of age. (Haun et al. 17572).

At first sight, this might seem like quite a blow for embodiment theories in Cognitive Science and Cognitive Linguistics who see embodied, egocentric experience as our primary way of making sense of the world.
But as Dirven et al. (2007) point out, “given the universality of human bodily experience,” it would not be “astonishing” if corporeal deixis constituted “the default case” of spatial cognition,
“but as a more refined conception of embodiment, the notion of situated embodiment incorporates and integrates man’s physical and social environment in his or her holistic bodily experience” (Dirven et al. 2007: 1217).


References:

Bühler, Karl. 1982. Sprachtheorie: Die Darstellungsfunktion der Sprache. Stuttgart,
New York: Fischer (Uni-Taschenbücher 1159).

Dirven, René, Hans-Georg Wolf, and Frank Polzenhagen. 2007. “Cognitive Linguistics and Cultural Studies.” In: The Oxford Handbook of Cognitive Linguistics, ed. by Dirk Geeraerts and Hubert Cuyckens. Oxford: Oxford University Press: 1203-1221.

Haun, Daniel B. M., Christian J. Rapold, Josep Call, Gabriele Janzen, and Stephen C. Levinson. 2006. “Cognitive Cladistics and Cultural Override in Hominid Spatial Cognition.” In: PNAS 103: 17568–17573.

Levinson, Stephen C. 2003. Space in Language and Cognition: Explorations in Cognitive Diversity. Cambridge: Cambridge University Press.

Levinson, Stephen C., Sotaro Kita, Daniel B.M. Haun, Björn H. Rasch. 2002. “Returning the Tables: Language Affects Spatial Reasoning.” In: Cognition 84: 155–188.

Palmer, Gary B. 2007. “Cognitive Linguistics and Anthropological Linguistics.” In: The Oxford Handbook of Cognitive Linguistics, ed. by Dirk Geeraerts and Hubert Cuyckens. Oxford: Oxford University Press. 1045-1073.

Pederson, Eric. 2007. “Cognitive Linguistics and Linguistic Relativity.” In: The Oxford Handbook of Cognitive Linguistics, ed. by Dirk Geeraerts and Hubert Cuyckens. Oxford: Oxford University Press. 1012-1044.

Talmy, Leonard. 1983. “How Language Structures Space.” In: Spatial Orientation: Theory, Research and Application. ed. by Herbert L. Pick, Jr., and Linda P. Acredolo. New York: Plenum Books. 225–82.

Thursday, June 18, 2009

Studying the Evolution of Cognition and Language: Are We Wasting Our Time? (Part 2)

In my last post I discussed some of the criticisms faced by people interested in the evolution of cognition.
One of the harshest critics is Richard Lewontin, who, at the end of his article "The Evolution of Cognition: questions we will never answer", advises his readers to “
to give up the childish notion that everything that is interesting about nature can be understood. History, and evolution is a form of history, simply does not leave suffcient traces, especially when it is the forces that are at issue. Form and even behavior may leave fossil remains, but forces like natural selection do not. It might be interesting to know how cognition (whatever that is) arose and spread and changed, but we cannot know. Tough luck.. (Lewontin, 1998: 130).”
But what leads Lewontin to conclude his essay in such as pessimistic and definitive manner?
According to Lewontin, there are three main strains of evolutionary explanations. And with each strain there are problems with evolutionary inquiries into cognition.

Historical Explanations
Firstly, there is a strain that explains the patterns of similarities and differences between animals through historical relatedness. Humans, for example, are more similar to and share more traits with chimpanzees than with lemurs because the human/chimpanzee lineages split some 5-7 million years ago and the lemur/human lineage split some 78 million years ago.

Functional Explanations
Secondly, there is a strain that tries to explain these patterns by looking at the functions they perform and the adaptive advantage they may have. The bodily similarities of sharks, dolphins, seals, and penguins for example can be explained by the fact that their bodies are adapted to swimming in the sea. Similarly, the differences between closely related species can be explained by adaptations to different environments. The differences between cows, goats, and deer, for example, only arose in the last 10 million years due to the different environments they had to adapt to. (Lewontin 1998: 116).

Problems for Studying the Evolution of Cognition
This is of course a problem for studying the evolution of cognition. Chimpanzees are the closest relatives that still exist but we and them may both have diverged so far from our ancestors that studying the cognitive differences between us may not really give us an insight into much human evolution. Indeed, there even is a study claiming “
more genes underwent positive selection in chimpanzee evolution than in human evolution.” (Bakewell et al. 2007).
Overall,
“Humans and chimpanzees are nevertheless very similar in their proteins, on the average, but vastly different in the sizes of their brains and their ability to write books about each other.” (Lewontin, 1998: 117).
But here is a point where I disagree with Lewontin: the research shown earlier indeed indicates that there probably was not a large amount of changes in brain-related genes that led to human cognition:
“This conclusion, however, does not preclude the possibility that substantial accelerations occurred in the evolution of a few nervous system genes during human origins. Indeed, several such examples are known, including genes that control brain size and speech development. (Shi et al. 2006).
And indeed, a recent article based on assumptions similar to that of these researchers and Lewontin, by Derek Penn and his colleagues, (2008) doesn’t see things so negatively as Lewontin but instead sees these considerations as offering a great chance.

If there really is “profound functional discontinuity between human and nonhuman minds” we can ask if there is a core ability that is responsible for it.
For Penn et al. psychological, comparative and developmental studies point towards the conclusion that this cognitive cap
“is largely due to the degree to which human and nonhuman minds are able to approximate the higher-order, systematic, relational capabilities of a physical symbol system.”
Sara Shettleworth (2009), in her critique of Bolhuis & Wynne’s (2009) arguments which are quite similar to that of Lewontin, agrees that
“There is evidence from behavioural studies that many of humans' mental powers are shared by other animals, including simple forms of learning, memory and categorization, and the elements of social, spatial and numerical cognition.
Only against this background does it make sense to propose, as some have, that there is a distinct small set of mental powers that is unique to humans […].”
Other researchers also defend the view that, contrary to Lewontin, we can learn a lot about the evolution of primate and human cognition by comparing different extant species. Jonathan Kenneth Burns (2004), for example, directly attacks Lewontin's arguments in an article on the evolution of Schizophrenia by stating that primatologist Richard Byrne
“has listed the establishing of a reliable pattern of descent as one part of a methodology for inferring the history of primate cognition (Byrne 2000). Many authors have confirmed the close evolutionary relationship between simian and ape species and modern Homo sapiens, with strong data from comparative psychology, molecular biology, and physical anthropology. Thus, cladistic analysis provides us with living relative species with which we can test the hypothesis that there is a heritable variation for social cognition that increases fitness.“ (Burns 2004: 868)
Evolutionary Constraints
But back to Lewontin’s article. The third strain of evolutionary theory he mentions is the one focusing on developmental and physiological constraints in the evolution and development of organisms. In the billion years of vertebrate evolution, for example, no organism ever developed more than four limbs.
Equally, mammals that went back into the sea and became whales and seals, the turned their limbs into flippers and flukes, but still retained their basic mammalian skeletal architecture.
This probably means that there are basic biological constraints because the available material regulates which evolutionary changes are possible, although the functions and activities of organisms and their parts may change quite dramatically over evolutionary time.
It also implies that
“when new functions arise in evolutiom, they often do so through a process of recruiting previously existing organs or physiological activities.” (Lewontin 1998: 117).
But If a trait is unique to one species it may be that we can’t really find any direct precursors and that it thus has no real “observable evolutionary history.”
What is more, we can’t be sure if a similar trait in other species it is far from clear if
"we are dealing with the same trait in the genetic, anatomical, and physiological sense.” (Lewontin 1998).
Platforms for the evolution of human cognition
I would argue however, that studies that show that similar cognitive activities which activate and rely on similar neural systems are a strong candidate for homologous platforms for human cognitive evolution. In fact, we now know that there are strong neural similarities between aspects of the macaque conceptual system and the human once (Gil-da-Costa et al. 2004).
With research like this we can thus probe into the “common architecture” that “underlies the conceptual systems of different species”, and ask how “additional systems” may have extended “human conceptual abilities significantly” (Barsalou 2005).
We also know now that “Communicative Signaling Activates ‘Broca’s’ Homolog in Chimpanzees,” and recent comparative neuroimaging studies have given new and important insights into the evolution of specialized language areas in human evolution. (for a great summary see this post).

Concluding Remarks
These examples lead me to think that we can learn a lot about the evolution of human cognition and language if we draw together the massive amount of data on the subject from all the different disciplines in a coherent and sensible manner. We simply have much more data to work with than at the time Lewontin voices his criticisms. Studying the evolution of cognition is – or has become – more than a ‘Paleofantasy’ in which we simply tell stories because we don’t know enough. Quite to the contrary – often it is the incredible wealth of data from different disciplines that presents the biggest problem.
Sverker Johansson's (2005) gargantuan collection of data relevant to the study of language evolution bears testament to this. The Study of language evolution, after it has moved beyond its ‘adaptationist’ beginnings in the early to mid-nineties – which Lewontin rightly criticized in some respects – is still a developing and growing field and I certainly agree with Willem Zuidema (2005) who states that
“Only when we have precise scenarios of the evolution of language and worked out ways to test empirically the plausibility of one scenario against another, can we conclude . if that turns out to be the case that there are too many alternative scenarios consistent with the available data. In my view, we have certainly not reached this stage yet.”


I hope I can wrap up my discussion of Lewontin's article next week.

References:

Bakewell,Margaret A., Peng Shi, and Jianzhi Zhang (2007:) More genes underwent positive selection in chimpanzee evolution than in human evolution. PNAS 104: 7489-7494.

Barsalou, Lawrence W. 2005. “Continuity of the conceptual system across species.” Trends in Cognitive Science 9.7: 309-311.

Bolhuis, Johan and Clive D. L. Wynne (2009):Can evolution explain how minds work?' Nature 458: 832–833.

Burns, Jonathan Kenneth. (2004) An evolutionary theory of schizophrenia: Cortical connectivity, metarepresentation, and the social brain. Behavioral and Brain Sciences
27(6):831–55; Discussion, 855–85.

Byrne, Richard W.(2000) Evolution of primate cognition. Cognitive Science 24(3):543–70

Gil-da-Costa, Ricardo, Allen Braun, Marco Lopes, Marc D. Hauser, Richard E. Carson, Peter Herscovitch and Alex Martin. 2004. “Toward an evolutionary perspective on conceptual representation: Species-specific calls activate visual and affective processing systems in the macaque.” PNAS 101.50: 17516–17521.

Johansson, Sverker (2005): Origins of Language: Constraints on Hypotheses. Amsterdam: Benjamins.

Lewontin, R. C. (1998) The evolution of cognition: Questions we will never answer. In D. Scarborough and S. Sternberg, editors, An invitation to cognitive science, Volume 4: Methods, models, and conceptual issues. Cambridge, MA: MIT Press

Shettleworth, Sara J. (2009). Cognition: theories of mind in animals and humans. In: Nature 459: 506.

Shi, Pen Margaret A. Bakewell and Jianzhi Zhang(2006):Did brain-specific genes evolve faster in humans than in chimpanzees? Trends in Genetics 22: 608-613.
Monday, June 15, 2009

Studying the Evolution of Cognition and Language: Are We Wasting Our Time? (Part 1)

This is my penultimate post in my short series on human uniqueness (1, 2, 3).

In a recent article in nature, Johan J. Bolhuis and Clive D. L. Wynne asked “Can evolution explain how minds work?” (subscription needed) and were of the opinion that there are severe problems with comparative paradigms. They pointed out major problems with evolutionary interpretations of cognitive traits. In their view, this research was fraught with anthropocentrism, e.g. it was mostly focused on humans or seen from a human perspective, and it doesn’t take into account the problem of convergent evolution:

“Different species may have arrived at similar solutions to cognitive problems because they have experienced similar selection pressures, not because they are closely related. In other words, evolutionary convergence may be more important than common descent in accounting for similar cognitive outcomes in different animal groups” (Bolhuis & Wynne 2009).


In addition, we don’t know which selective pressures our ancestors faced in their environment. Cognitive traits also leave little to no traces in the fossil record. This means that we mainly have to guess which cognitive traits may have evolved in response to some presumed selection pressures.


Bolhuis and Wynne also hold that comparative researchers have “naïve evolutionary presuppositions” and hold that

“As long as researchers focus on identifying human-like behaviour in other animals, the job of classifying the cognition of different species will be forever tied up in thickets of arbitrary nomenclature that will not advance our understanding of the mechanisms of cognition.” (Bolhuis & Wynne 2009).


This argument is of course not new and can be found – in an even stronger form and on a more general level – in the critical writings of Noam Chomsky, Stephen Jay Gould, and maybe most vocally, Richard Lewontin. Lewontin even goes so far as to say that the only thing we know about the evolution of human cognition is precisely that it evolved. That’s it. (Lewontin 1998: 108). This is especially so with complicated cognitive traits like linguistic competence.


We don’t even know in how far language is an innate genetically specified ability and in how far it is only a by-product of other evolutionary changes and is shaped and specified by culture. What’s more, we can’t possibly know how hereditary mechanisms (both genetic and cultural) acted in our remote ancestor, and we don’t know anything about the survival advantage these presumed mechanisms may have had in the past. Lewontin draws the conclusion that “reconstructions of the evolutionary history and the causal mechanisms of linguistic competence […] are nothing more than a mixture of pure speculation and inventive stories.” (Lewontin 1998: 111).

He explicitly directs his criticism at proposals like that of Pinker & Bloom (1990) (see also this post) who argued that natural selection is the only force that can explain the evolution of such a ‘complex adaptive’ trait like language. But we can’t show how natural selection might have been at work in each of the unknown stages that were necessary for language to evolve. Consequently, Pinker & Bloom’s argument is flawed.


I think Lewontin’s argument applies to some of the sweeping ‘adaptationist’ evolutionary approaches to language and cognition. But I don’t think his 1998 critique really captures the state of the research today or even earlier. In the 2003 anthology ‘Language Evolution’ (Kirby & Christiansen 2003, see also this post) which pretty much presented the state of the field there were many researchers who had a substantial amount to say about the evolution of language without falling into the theoretical pitfalls Lewontin warned about. At the end of his article Michael Tomasello, for example, cautions that “I am afraid that I have no real evolutionary fairy tale with which to conclude.” But he still has to clarify what valuable implications his research has for a general account of the evolution of language and cognition and is able to spell out some of the cognitive mechanisms which had to evolve and in how far culture has been an important aspect in this respect (Tomasello 2003: 108f.). Similarly, Marc Hauser and W. Tecumseh Fitch voice similar criticism to that of Lewontin and Chomsky (which is not very surprising given that they co-authored two papers with the latter). However, they hold that the “comparative approach to language has been and will continue to be a powerful approach to understand both the evolution and current function of the language faculty.” (Hauser & Fitch 2003: 159). I completely agree with them, especially if we throw developmental science into the mix. By looking at non-human primates we are able to “isolate and study those components of the language faculty inherited from our non-human ancestors” (Hauser & Fitch 2002: 159). What is more, comparative research can also give us insight into possible advantages and selection pressures that led to the evolution of features. If we find similar traits and neural subsystems in other primates it is reasonable to assume that these are homologous and due to our shared evolutionary history. If on the other hand, other primates don’t have these traits but other species, e.g. songbirds, jays, parrots or deer, have them, they may be analogous and due to similar environmental or social selection pressures. If we carefully compare many different species across different taxa we get an increasingly better picture of the evolution of cognition in humans and other species.

But a broad survey of the field shows that this is already done as Sara Shettleworth (2009a) points out. Consequently, Bolhuis and Wynne’s criticism falls apart if we actually look at the field they are criticising and it is more as if they are flogging a dead horse (2009b). But we can see that Tomasello, Hauser, Fitch, Bolhuis, Wynne and Shettleworth all think that comparative cognition can give us important insights into the evolution of the organisms they study and compare. But it has to be done carefully and critically and within a throroughly worked out theoretical and methodological framework. In light of this, much of Lewontin’s criticisms seem to be misguided or at least do not really apply anymore. But does this really mean that there are no real general problems with evolutionary inquiries into the evolution of cognition?

In my next post I will address the additional criticisms Lewontin launches at the study of the evolution of cognition.


References:

Bolhuis, Johan and Clive D. L. Wynne (2009):Can evolution explain how minds work?' Nature 458: 832–833.

Hauser, M. D. & Fitch, W. T. (2003). What are the uniquely human components of the language faculty? In: Language Evolution: The State of the Art. Ed. by Christensen, M. & S. Kirby) pp. 158-181. Oxford: Oxford Unviersity Press.

Normal 0 21 Lewontin, R. C. (1998) The evolution of cognition: Questions we will never answer. In D. Scarborough and S. Sternberg, editors, An invitation to cognitive science, Volume 4: Methods, models, and conceptual issues. Cambridge, MA: MIT Press

Pinker, Steven & Paul Bloom (1990): “Natural Language and Natural Selection.” In: Behavioral and Brain Sciences 13.4: 707-726.

Shettleworth, S. J. (2009a). The evolution of comparative cognition: Is the snark still a boojum? In: Behavioural Processes , 80, 210-217.

Shettleworth, Sara J. (2009b). Cognition: theories of mind in animals and humans. In: Nature 459: 506.

Tomasello, M. (2003). On the different origins of symbols and grammar. In Language Evolution: The State of the Art. Ed by. M. Christiansen & S. Kirby. Oxford: Oxford University Press.

Tuesday, June 9, 2009

Michael Tomasello - Why We Cooperate

Michael Tomasello has a new book out in October called "Why We Cooperate." What is interesting about this publication is that Tomasello presents his findings on great ape and infant cognition and and social and developmental psychologist Carol Dweck, anthropologist Joan Silk, philosopher Brian Skyrms, and developmental psychologist Elizabeth Spelke respond to and explore the implications of his work in light of their own research.

Here's the description:

"Drop something in front of a two-year-old, and she's likely to pick it up for you. This is not a learned behavior, psychologist Michael Tomasello argues. Through observations of young children in experiments he himself has designed, Tomasello shows that children are naturally—and uniquely—cooperative. Put through similar experiments, for example, apes demonstrate the ability to work together and share, but choose not to.

As children grow, their almost reflexive desire to help—without expectation of reward—becomes shaped by culture. They become more aware of being a member of a group. Groups convey mutual expectations, and thus may either encourage or discourage altruism and collaboration. Either way, cooperation emerges as a distinctly human combination of innate and learned behavior.

In Why We Cooperate, Tomasello's studies of young children and great apes help identify the underlying psychological processes that very likely supported humans' earliest forms of complex collaboration and, ultimately, our unique forms of cultural organization, from the evolution of tolerance and trust to the creation of such group-level structures as cultural norms and institutions.

Scholars Carol Dweck, Joan Silk, Brian Skyrms, and Elizabeth Spelke respond to Tomasello's findings and explore the implications."

Thursday, June 4, 2009

Some Links

The Exploratorium (in San Francisco) and the Max-Planck-Institute for Evolutionary Anthropology have a nice site up called "Exploratiorium Evidence: How Do We Know What We Know?"

"Science is an active process of observation and investigation. Evidence: How Do We Know What We Know? examines that process, revealing the ways in which ideas and information become knowledge and understanding.
[...]
In this case study in human origins, we explore how scientific evidence is being used to shape our current understanding of ourselves: What makes us human—and how did we get this way?"
Hat-tip: Afarensis

Sandy G of The Mouse Trap also has a nice post up called "What is it like to be a zombie?"

Also, Ed Yong of Not Exactly Rocket Science reports on research which found that Chimps use Swiss army toolkit to rob beehives
I find the possible implications of the fact that chimpanzees use several multi-functional tools for honey-extraction quite fascinating.
As I've written before (see also this post), linguists like Dieter Wunderlich argue that the ability to change an existing structure and then further work on the qualitatively changed output in a hierarchical, recursive, and compositional manner - as for example exemplified by crafting hand axes - is a precursor to or even the same process athis the compositionality found in language. If chimpanzees are able ts io work with and modify tooln a compositional manner this would provide another insight into the possible cognitive platform from which language evolved.

Monday, June 1, 2009

The Nature and Evolution of Human Cognition: Considerations from Comparative and Developmental Psychology


If we bear in mind the proposals for what (among other things) makes human cognition unique I summed up in my last post – along with the conjecture that our cognitive style may more be something of a idiosyncrasy due to a highly specific cognitive specialization instead of a definitive quantitative and qualitative advance over other styles of animal cognition, we can look for studies which further point in that direction.

Chimpanzees, for example, beat humans at certain memory tasks (Inoue & Matsuzawa 2007) and behave more rational in reward situations (Jensen et al. 2007). In addition, it has been shown that in tasks in the social domain, which are generally assumed to be cognitively complex, domesticated animals such as dogs and goats (Kaminski et al. 2005) fare similarly well or even outperform chimpanzees. It is entirely possible that the first signs of human uniqueness where first simply side-effects our self-domesticating lifestyle – the same way the evolution of social intelligence in dogs and goats is hypothesised to have come about –, acting on a complex primate brain (Hare & Tomasello 2005).

It is certainly a fact

“that Homo sapiens has become ‘localized’ by having to depend upon learned, culture-specific modes of interacting.” (Bruner 2005: 693).
Humans are constantly immersed in culture and social interactions and at the same time extremely dependent on it, and human ontogeny fundamentally differs from that of any other primate species. Human infants are even more helpless and completely dependent on others, and remain unable to feed and care for themselves for a uniquely long time span. Furthermore, childhood and adolescence are two additional and prolonged states of mental development and cultural learning absent in any other species that seem to be vitally important for the development of culturally adept and cognitively highly sophisticated human beings (Locke & Bogin 2006).

The fact that social interaction, learning, and cultural transmission play such a vital and important role for children’s ongoing cognitive development indicates that hey have a biologically-based “adaptation for culture” which has to be operative from early on. Comparing young children’s and infants cognitive abilities with that of the other great apes may be a useful indicator of the biological foundations of what makes us uniquely human. In Addition, we can gain crucial insights on what platform the evolution of human cognition could have started because chimpanzees are “conservative species” that has always lived in tropical forests, which is why they didn’t have to change as much as we did to adapt to fundamentally new environments and selection pressures. This also means that chimpanzees are more similar to the last common ancestor we shared with them than we are (Gazzaniga 2008: 51).

If we now compare the performance of 2.5 year-old children and other great apes (in this case chimpanzees and orangutans) across a wide range of domains we indeed find that in some domains the differences are much more marked than in others. (see also, this post). In the physical domain, which includes the understanding of space, quantity and causality, the subjects were tested by rewards that were out of reach and could only be retrieved with a stick (causality), or had to locate a reward that was not directly accessible but had to be located (space). In the social domain, subjects had to follow “an actor’s gaze direction to a target,” solve “a simple but not obvious problem by observing a demonstrated solution” (social learning), or understand what an actor intended to do, but in the end failed to. (Intention attribution or Theory of Mind).

Generally, orangutans fared worst in most of the test, whereas chimpanzees and humans were quite similar in the physical domain. In some of the physical tasks, especially the one which required active tool use, chimpanzees even out performed human children. But in the causality tasks in which

“a judgment must be made before manipulation or choice” (Hermann et al. 2007:1362)
children were better. They were also better in inhibitory and cognitive control in general, something that is expected given what we know about the disproportionate dominance and prominence of higher-order prefrontal circuitry, which better enable a child’s brain
“to coordinate processing among its millions of neurons in order to direct them toward future goals.” (Miller et al. 2002: 1131)
than is the case in other great apes. According to the research group that did these experiments

“the current results provide strong support for the cultural intelligence hypothesis that human beings have evolved some specialized social-cognitive skills (beyond those of primates in general) for living and exchanging knowledge in cultural groups: communicating with others, learning from others, and “reading the mind” of others in especially complex ways“ (Hermann et al. 2007: 1365).

But as indicated by children’s performances in the causality task, and in congruence with the models of human cognition I’ve outlined above, the social domain is not the only catch-all distinctive property of human minds. Instead, the ability to re-interpret cognitive data in terms of more abstract properties such as “unobserved causal forces” and “mental states” seems to be distinctive foundation for excelling performances in both the physical and social domains. The authors find it plausible however, that

"understanding hidden causal forces evolved first to enable humans to understand the mental states of other persons, and this generalized only later to the physical domain.”

This is why we are justified in further looking for uniquely human attributes in the socio-cognitive development of children.


References:


Normal 0 21

Bruner, Jerome (2005): “Homo Sapiens, a localized species”. In: Behavioral and Brain Sciences 28:5, 694–695.


Gazzaniga, Michael S. (2008): Human: The Science of What Makes us Unique. New York: Harper-Collins.

Hare, B., & Tomasello, M. (2005). Human-like social skills in dogs? Trends in Cognitive Science, 9, 439-444.


Hermann, Esther, Josep Call, María Victoria Hernández-Lloreda, Brian Hare, and Michael Tomasello. 2007. “Humans Have Evolved Specialized Skills of Social Cognition: The Cultural Intelligence Hypothesis” Science 317: 1360-1366.


Inoue S. and T. Matsuzawa (2007). Working memory of numerals in chimpanzees. Current Biology, 17(23), R1004-R1005.


Jensen, Keith, Josep Call and Michael Tomasello (2007): Chimpanzees Are Rational Maximizers in an Ultimatum Game. Science 318: 107-109


Kaminski, Juliane, Riedel, J., Call, J. & Tomasello, M. (2005) Domestic goats (Capra hircus) follow gaze direction and use social cues in an object choice task. Animal Behaviour, 69(1), 11-18.


Locke, John L. and Barry Bogin. (2005) “Language and life history: A new perspective on the development and evolution of human language” Behavioral and Brain Sciences 29, 259–325.


Miller, Earl K., David J. Freedman and Jonathan D. Wallis (2002.) “The Prefrontal Cortex: Categories, Concepts and Cognition.” In: Phil. Trans. R. Soc. Lond. B 357: 1123–1136.